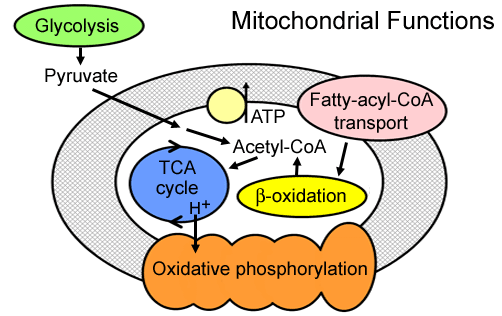
I've held off on posting this for a while because it's a screen shot and I have no idea whom to credit. But, since the metabolic pathways are common knowledge, I've decided there's no real harm done "publishing" any depiction of them on my li'l old blog. (If anyone recognizes the graphic, please notify me so I can extend credit)
An enduring point of controversy exists in the LC community over higher protein intake vs. higher fat. My personal experience is that the former works for me, but there are plenty of folks doing well on high fat controlled protein approaches.
One of the advocates of lower protein intake is Dr. Bernstein the diabetes specialist. Most that advocate his approach agree with his central premise that excess protein is converted to sugar or metabolized as such. While theoretically possible, I've been doing some "re-educating" of myself where protein metabolism, specifically what becomes of any excess is concerned.
OK, so here it is:
This is the most concise depiction of the various amino acids and where they can feed into metabolic pathways. The "green boxed" AA's are termed glucogenic AA's because they can be turned into glucose under certain conditions. The "white boxed" AA's are ketogenic as they cannot be converted to glucose entering the metabolic paths at these junctures. You will note that certain AA's are potentially ketogenic or glucogenic because they can be converted to different substrates.
The blue-arrowed cycle here is the Citric Acid Cycle, aka Kreb's Cycle. Of note is that the central linking molecule of carb and fat metabolism, Acetyl CoA, is the primary "external substrate" feeding into this cycle (black arrow). The primary substrate for glucose formation (gluconeogenesis) is oxaloacetate -- the last "stop" on the cycle. Pyruvate is the product of glycolysis -- glucose metabolism -- but it's both a product and substrate for other metabolic pathways.
The pink arrows are gluconeogenesis (and we know there's also glyceroneogenesis from pyruvate). However my research points to these pathways being stimulated in response to the carbohydrate restriction component of fasting and not to amino acid levels although that might be possible. This seems to be the concensus in the LC community as well -- our bodies will only turn protein to glucose to meet needs. Some of the excess may be "burnt like sugar" because it enters the Krebs Cycle by going through the pyruvate pre-cursor, but this really just means another step to get to the ultimate central molecule of Acetyl CoA.
So, excess protein gets used for energy like ... well ... excess amino acids (as opposed to glucose or fatty acids). Or if you want to get semantically picky, some feed into metabolic pathways involving glucose, and some into pathways for fatty acids, and some like neither of the other macronutrients. Too much available energy from any source and Acetyl CoA gets converted to fatty acids -- de novo lipogenesis! In this regard, protein would be the least lipogenic of the macronutrients. For a while there I was under what I now realize to be an incorrect assumption, that protein-to-fat would go through glucose to AcCoA to fatty acid by DNL. But this seems an unlikely path except, perhaps, in the diabetic with issues of over-active gluconeogenesis. Still, I'm unsure if that path would be further enhanced simply by an excess of pyruvate and/or oxaloacetate made available by excess AA's.
Limiting protein for weight loss does not seem to be a very good strategy unless someone wants to lose muscle mass, particularly for someone consuming a VLC diet. The VLCer's body will make glucose and get the necessary AA's from where it will -- better the diet than the body IMO. Protein is almost impossible to overeat. For diabetics, however, relying on protein as an energy source may present other issues as relates to various complications of that disease.
Previously I've characterized protein as a poor energy source. However, I no longer believe this to be true. It is not a preferred energy source, perhaps, but it seems to feed pretty efficiently into Krebs.